High-Efficiency Transformation of Yeast
Written by Isreal
Introduction:
The CDC42 gene or Cell Division Control 42 gene has homologies in many species ranging from yeast to humans. This gene controls and influences many pathways that are important in the formation of many proteins. One of the great things about CDC 42 is that we can use a mutated strain and, through transformation, actually change the genetic material within the cell (Ito, Fukuda, Murata, and Kimura, 1983). This would cause complementation within the cell. Transformation is the exchange or uptake of genetic material, which ultimately changes the genetics of any given cell.
Transformation is being widely studied because it could result in many cures and breakthroughs in the medical field. In this lab in particular, we are looking at the transformation of a cdc42ts strain of yeast. This strain has a mutation in the CDC42 gene that causes the cells to be unable to grow at higher temperatures as well as another mutation at another point on the genome that inhibits the production of leucine. By using polyethylene glycol (PEG), lithium acetate (LiAc), and a single stranded carrier DNA (from salmon sperm) it is possible to introduce two different plasmids (pPGK2E and pPGK2ECDC42) into the mutated yeast strain. The results of this transformation is complementation that allows both strains to grow on plates lacking leucine (Leu–) and one strain to grow at a non-permissive temperature (37°) while the other die.
Editor’s note, November 2026: Lithium acetate wording and leucine/Leu spellings have been corrected, and a short explanation of complementation and replica plating is added against Tables 1 and 2. The first-paragraph citation has been corrected to Ito, Fukuda, Murata, and Kimura, 1983. The 2010 reference is identified below as Ito et al., J. Clin. Invest., a mouse Cdc42 study, not a yeast-transformation methods paper. A fish-DNA-in-plants example cited to Ivics et al. 1997 has been removed; that paper does not support the claim.
Materials and Methods:
There was a deviation from the protocol that was outlined in the lab (Burke, et al 2000). Instead of having three plates, we only had two due to the lack of available plates. We obtained our data for the water control plate from the class. This procedure also called for the use of the sterile bead technique to plate the control and each transformation. Each plate contained SC-Leu– for the purpose of selecting only the cells that took in the plasmids to grow. This media was used to demonstrate the ability of the transformed yeast to grow on Leu– plates at a permissive temperature, since one of the mutations that this strain of yeast has is the inability to make its own leucine. The media, through the water control plate, shows that the original strain is in fact Leu–. To test for temperature sensitivity, the plates must be replicated using a replicating block from VWR Scientific Company and grown at a non-permissive and permissive temperatures.
Results:
|
Water control |
pPGK2ECDC42 |
pPGK2E |
|
0 |
720 |
1348 |
Table 1. Transformation of Yeast Results. The plates were made by using the sterile bead technique and allowed to grow for three days at 30°. This data shows that the strain of yeast did in fact take in the pPGK2ECDC42 and pPGK2E plasmids. It also shows that the original strain cannot grow on plates lacking leucine.
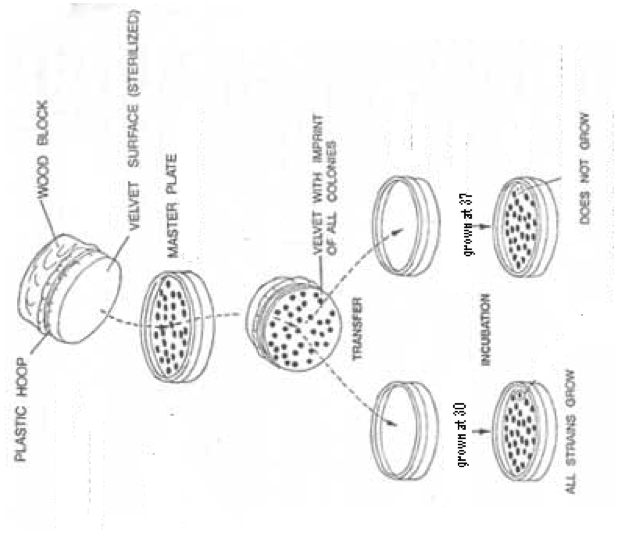
Figure 1. Technique for Replicating Plates. This diagram demonstrates how to perform the technique of replica plating. This is done for each of the two strains of transformed yeast. The first plate to be replicated must be the one to be exposed to 37°.This diagram pictures the pPGK2E strain. This strain is temperature sensitive and cannot grow at the non-permissive temperature of 37°.
|
Temp. |
pPGK2ECDC42 |
pPGK2E |
|
30° |
+ |
+ |
|
37° |
+ |
– |
Table 2. Replica Plate Results. The replicated plates were grown for three days at two temperatures: at a non-permissive 37° and at a permissive 30°. The results above show that the pPGK2E lacks the ability to grow at higher temperatures, while pPGk2ECDC42 has the ability.
The data in Table 1 and Table 2 show the complementation that has occurred between the mutant cdc42ts yeast strain and the two plasmids. Table 1 shows that both of the plasmids contain the ability to produce leucine, allowing them to grow on the Leu– plates. Table 2 shows that only the pPGK2ECDC42 complements the mutant yeast, giving it the ability to grow at the non-permissive temperature while the pPGK2E lacks this ability.
The untransformed cdc42ts strain cannot make leucine and cannot grow at 37°C. Table 1 records colony counts on SC-Leu– plates after three days at 30°C: 0 for the water control, 720 for pPGK2ECDC42, and 1348 for pPGK2E. The water-control count of 0 shows that the original strain is a leucine auxotroph and cannot form colonies on medium lacking leucine. Growth of both plasmid-treated cultures on the same medium shows that each plasmid supplies a function that restores leucine prototrophy, which is the selectable marker for cells that took up a plasmid.
Replica plating transfers the colony pattern from a master plate onto fresh plates with a sterile replicating block, so the same colonies can be scored under more than one condition (Lederberg and Lederberg, 1952). Figure 1 illustrates that transfer. Table 2 reports growth after the replicas were incubated for three days at 30°C and at 37°C: both plasmid strains grow at the permissive temperature of 30°C, but only pPGK2ECDC42 grows at the non-permissive temperature of 37°C. That pattern means pPGK2ECDC42 complements the cdc42ts mutation, consistent with the plasmid name and with the report’s own reading of Table 2, while pPGK2E does not. Complementation here is the restoration of a missing host function by a wild-type gene introduced on a plasmid; it is scored by the leucine selection in Table 1 and by temperature in Table 2.
Discussion:
The first part of this lab was to show the uptake of the plasmid DNA by a cdc42ts strain of yeast. This strain is mutated so that it will die at non-permissive temperatures. Lithium acetate, PEG, and single-stranded carrier DNA were all used and each improves uptake of the plasmid DNA by intact yeast cells. Lithium acetate does not puncture the cell wall. In the usual description of this method, PEG is required for plasmid DNA to attach to the cell surface, and lithium acetate (with the brief heat shock used in the protocol) helps that DNA cross the cell wall of intact cells; how the DNA then reaches the nucleus is not fully settled (Kawai, Hashimoto, and Murata, 2010). Single-stranded carrier DNA, often from salmon sperm, further increases transformation efficiency, likely by improving plasmid binding at the cell surface; its exact role is still not completely defined. The results of this first part of the experiment showed complementation occurring. The plasmid DNA complemented the yeast cell, making it capable of producing its own leucine thus growth was seen on the SC-Leu– plate. Showing that both strains grow on the Leu– plates, it is possible to now determine any temperature sensitivity that remains. Since the original strain had a mutation on CDC42 that caused it to be temperature sensitive, any growth at the non-permissive temperature would be proof of complementation. The results confirmed this. At the non-permissive temperature, the pPGK2E strain died while the pPGK2ECDC42 experienced growth.
The results of this lab show, through transformation, that complementation has occurred between the introduced plasmids and the yeasts’ own DNA.
References:
Burke, Dan, et al. Methods in Yeast Genetics. Cold Spring Harbor Laboratory Press. 2000 edition.
Ito, H., Fukuda, Y., Murata, K., and Kimura, A. (1983). Transformation of intact yeast cells treated with alkali cations. J Bacteriol 153(1), 163-168. doi:10.1128/jb.153.1.163-168.1983.
Ito, Y., Teitelbaum, S.L., Zou, W., Zheng, Y., Johnson, J.F., Chappel, J., Ross, F.P., and Zhao, H. (2010). Cdc42 regulates bone modeling and remodeling in mice by modulating RANKL/M-CSF signaling and osteoclast polarization. J Clin Invest 120(6), 1981-1993. doi:10.1172/JCI39650. (Previously listed under the misspelled lead author “Chapoel, J.”; Jean Chappel is a co-author. This is a mouse osteoclast study, not a yeast-transformation methods paper, and it is a different Ito from the 1983 lithium-acetate methods paper.)
Kawai, S., Hashimoto, W., and Murata, K. (2010). Transformation of Saccharomyces cerevisiae and other fungi: methods and possible underlying mechanism. Bioeng Bugs 1(6), 395-403. doi:10.4161/bbug.1.6.13257.
Lederberg, J., and Lederberg, E.M. (1952). Replica plating and indirect selection of bacterial mutants. J Bacteriol 63(3), 399-406.